lecture 12
 Call Kai
 Learn
 Practice Test
 Spaced Repetition
 Match
 Flashcards
 Knowt Play
1/23

Earn XP
Description and Tags
Molecular Regulation Chapter 10
24 Terms
Introduction
A bacterial genome encodes thousands of different proteins needed to handle many types of environmental contingencies.
To compete successfully with others, and remain competitive the microbe will not waste energy making unneeded proteins.
- It uses elegant mechanisms to control gene expression at various levels.
- Transcription, posttranscription, translation, and post translation
Molecular Regulation
Many different proteins are needed to handle different aspects
¨“housekeeping proteins”: Essential proteins that the cell needs constantly just to stay alive and grow (often called constitutive proteins).
Always required for growth
¨Other proteins are only needed under a limited set of conditions:Specialized proteins that are only useful during specific situations or environmental stresses
Regulating Gene Expression
Cells use different mechanisms to sense and respond to conditions within or outside the cell.
Regulatory proteins help a cell sense internal changes and alter its gene expression to match the current environment.
Diagram:
Making the Regulatory Protein:
A specific gene on the DNA is transcribed and translated into a regulatory protein (the yellow circle).
Controlling the Target Gene:
This regulatory protein then travels to a specific regulatory sequence (the green block) on the DNA.
By binding there, it controls whether the nearby target gene gets expressed into structural proteins or enzymes
Operon vs Regulon
Top Diagram:
A. Operon (Top Diagram)
Operon A group of multiple related genes located right next to each other that are controlled by a single shared promoter.
Monocistronic vs. Polycistronic:
Monocistronic RNA: A single gene transcribed into its own separate mRNA molecule.
Polycistronic RNA: Multiple genes (Gene 1, Gene 2, Gene 3) transcribed together into one long strand of mRNA.
All these genes are turned on or off together as a single package.
B. Regulon (Bottom Diagram)
What it is: A collection of multiple separate operons or genes across the bacterial chromosome- controlled by the same single regulatory control protein.
How it works: When the cell senses a major environmental change (like acid stress or heat shock), the central control protein (yellow sphere) binds to all these scattered operons at once to turn them on or off simultaneously.
Summary
Operon: Local control — multiple genes right next to each other sharing one promoter.
Regulon: Global control — multiple operons spread all around the genome sharing one control protein.
so operon is one operon regulon is a bunch of them

Regulating Gene Expression
Regulatory proteins come in two forms:
- Repressors: Bind to regulatory sequences in the DNA and prevent transcription of target genes - Some must first bind a small ligand.
- Activators: Bind to regulatory sequences in the DNA and stimulate transcription of target genes - Most must first bind a small ligand.
Repressors vs activators
scenario 1: Induction (Removing the Repressor)
Default State: The repressor protein (red sphere) sits on the DNA by itself, blocking transcription.
Signal: A small ligand called an inducer (green diamond) binds to the repressor.
Result: The repressor pops off the DNA, allowing the target gene to be expressed.
Scenario 2: Derepression (Forming the Repressor Complex)
Default State: The repressor protein (yellow sphere) is inactive on its own and cannot bind DNA.
Signal: A small ligand called a corepressor (red triangle) binds to the repressor.
Result: The repressor-corepressor complex binds to the DNA, shutting down transcription. When the corepressor drops off, the repressor detaches and transcription resumes (derepression).

Repressors
Two types of repressors; those that: ‘
¨1) Bind operator DNA by themselves and prevent transcription
This repressor is naturally shaped to fit onto the operator DNA right away, acting like a roadblock that stops transcription by default.
To express target gene, an inducer (ligand) must bind to the repressor à causing it to release from the operator (induction)
¨2) Do NOT bind well to operator DNA unless corepressor (ligand) is bound
As the corepressor disappears, then corepressor is no longer able to bind to repressor
repressor releases from operator without corepressor
target gene can be expressed (derepression)
Activators
Activator proteins ¨Bind poorly to activator DNA sequences unless an inducer (a ligand) is present: Its in an idle state at this point
¨Once inducer binds to activator protein it can directly contact RNA polymerase molecule that is stuck at the nearby promoter: initiates transcription: The On switch stage
¨When the concentration of the inducer is low in the cell
the activator protein (without inducer) will leave the operator — therefore transcription is no longer activated
so basically
Idle, than inducer binds, than polymerase is recruited, than transcription starts, than inducer leaves transcription stops
The E. coli lac Operon
Jacques Monod and Francois Jacob
Lactose (milk sugar) is used for food ¨Cannot pass through plasma membrane
Lactose permease allows entry
It uses the Proton Motive Force (PMF)—a gradient of hydrogen ions across the membrane—as an energy drive to pull lactose inside
¨Must be converted to glucose to be digested
b-galactosidase converts lactose to glucose
¨ People also make B- galactosidase
¨ If not, person is lactose intolerant
Lactose Induces Expression of the lacZYA Operon
The lactose utilization lacZYA operon of Escherichia coli was the first gene regulatory system described.
First, here’s how lactose is transported and metabolized.
Diagram
Transport (Left): Lactose from the outside environment is pumped into the cell through a membrane channel protein called Lactose permease (LacY). Powered by proton motor force H+
The Inducer Signal (Top Right): Even when the operon is mostly inactive, a tiny, low-level amount of the enzyme beta- galactosidase converts a fraction of the incoming lactose into allolactose.
Allolactose is the critical chemical signal (the inducer) that will trigger the operon to turn on
Metabolism/Catabolism (Bottom Right): When fully expressed, high levels of beta-galactosidase chop lactose molecules apart into Galactose and Glucose, which the cell can directly burn for energy.
so the beta galactosidase that are already there make allolactose which acts as an alarm causing the operon to turn on and start making galactose and glucose
allolactose gets broken down into glucose and galactose too by B galactose

The E. coli lac Operon
The lacY gene encodes lactose permease
The lacZ gene encodes b-galactosidase
lacA: Encodes thiogalactoside transacetylase—an enzyme that detoxifies non-digestible galactosides that might sneak in along with lactose
Need both lacZ & lacY proteins to digest lactose
Operon ¨Multiple genes transcribed from one promoter ¨All genes are transcribed together
Shared Switch PLacZYA All three structural genes (lacZ, lacY, and lacA) sit right next to each other and share a single promoter (PLacZYA
Coordinated Expression: Because they share one promoter, all three genes are transcribed together into a single, polycistronic mRNA strand at the exact same time.
Operator region lacO: right next to the promoter acts as the binding site where the repressor protein attaches to block transcription when lactose isn't around.
so all 3 of the lac proteins are made at the same time

The Organization of the lacZYA Operon
Diagram
Two Separate Units: lacI and the lacZYA operon are separate transcriptional units, each with its own promoter. They are controlled independently
The Repressor Factory (lacI on the left):
The lacI gene has its own promoter PlacI
It is transcribed into its own mRNA, which is then translated into the LacI repressor protein (the red circle).
This gene is usually expressed at a steady, low level so the cell always has a supply of repressor proteins floating around.
The Target Operon (lacZYA on the right):
The repressor proteins produced by lacI float through the cell and bind to the operator (lacO) of the lacZYA operon, acting as the "brakes" to keep it locked and turned off when there is no lactose.

Scenario 1: Absence of Lactose
LacI binds as a tetramer to the operator region.
a tetramer is a cluster of four connected protein subunits
It represses the lac operon by preventing open complex formation by RNA polymerase.
DNA Looping (The Double-Grab)
Because it has multiple binding sites, the tetramer can grab onto two different operator regions on the DNA at the same time—specifically lacO and a secondary site called lacO1
forces the DNA in between them to bend and form a loop
3. Preventing Open Complex Formation
By clamping down and looping the DNA right over the promoter region, the repressor creates an impenetrable physical roadblock.
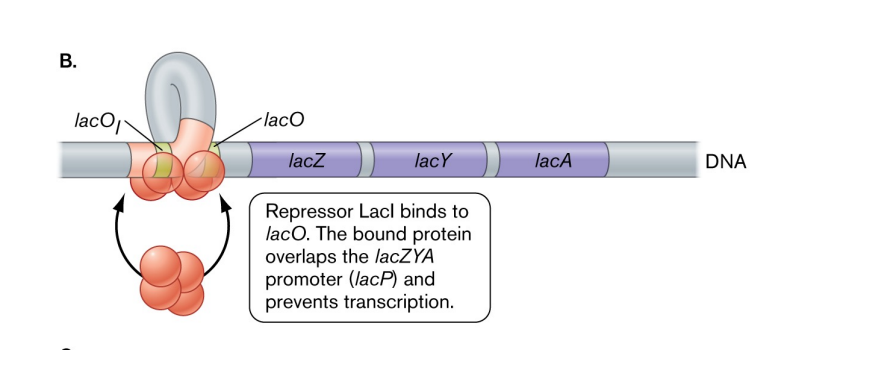
The Lactose Operon
Structure: the physical DNA loop created by the LacI repressor tetramer
The LacI Protein Clamp (Bottom): The multi-colored, four-part protein structure (the tetramer) sitting at the base as a heavy anchor
The Dual Grip (lacO and O1): The protein grabs the DNA strand at two separate locations simultaneously—one at the main lacO operator and another at the O1 site.
The DNA Loop (Top): Because the protein is holding onto two spots at once, it forces the DNA in between to balloon upward into a giant loop.
Trapped inside that loop is part of the promoter lacP.
so this happens when theres no lactose

Scenario 2: Presence of Lactose
b-galactosidase (LacZ), when at low concentrations, cleaves and rearranges lactose to make the inducer allolactose.
Allolactose binds to LacI which is the repressor , reducing its affinity to the operator and thus allowing induction of the lacO operator operon.
The clamp releases and transcription starts
The repressor pops off the DNA, breaking the loop. allows RNA polymerase to freely move down the line,
transcription of the operon occurs—flooding the cell with the mRNA needed to make all the digestion tools (lacZ, lacY, and lacA).
So theres lacI with italic I and LacI which is the repressor
Activation of Transcription by cAMP-CRP
Key Components
CRP (cAMP Receptor Protein): A regulatory protein that acts as an activator.
cAMP (Cyclic AMP): A small signaling molecule that acts as a hunger signal inside the cell (usually indicating a lack of glucose).
The cAMP-CRP Complex: When cAMP binds to CRP, they form a combined complex that can bind to the promoter region of the lac operon.
Maximum expression of the lac operon requires the presence of cAMP and cAMP receptor protein (CRP).
- The cAMP-CRP complex binds to the promoter, and interacts with RNA polymerase to increase the rate of transcription initiation
By holding onto RNA polymerase, it dramatically increases the rate at which transcription is initiated

Catabolite Repression
In catabolite repression, an operon enabling the catabolism of one nutrient is repressed by the presence of a more favorable nutrient (commonly glucose).
The biphasic curve of a culture growing on two carbon sources is often called diauxic growth.
Glucose is the favorite food: It’s a simple sugar that the cell can burn immediately without making any extra enzymes.
Lactose is the backup food: It requires extra effort because the cell has to make specialized tools beta galactosidase and lactose permease to break it down.
Pictures; Phase 1 (First Growth Curve - Glucose Utilized):
The bacteria grow rapidly by consuming all the available glucose. During this time, the lac operon remains completely repressed.
The Pause (The Flat Line):
Once the glucose completely runs out, growth stops temporarily. The bacteria hit a brief pause while they sense the empty glucose supply, spike their internal cAMP levels, and switch on the lac operon to start processing lactose.
Phase 2 (Second Growth Curve - Lactose Utilized):
Once the lac operon is fully activated, the bacteria resume growth at a steady rate by consuming the lactose until that runs out, too.
so basically growth than pause than growth

Catabolite Repression
Glucose transport by the phosphotransferase system (PTS) causes catabolite repression by inhibiting the LacY permease activity.
This is termed inducer exclusion.
A. Glucose Present (Top Panel: The Lockout)
The PTS System is Active: When glucose is available, the cell's glucose transport system (the phosphotransferase system, or PTS) actively pumps glucose inside using a chain of proteins (IIC, IIB, and IIA).
Unphosphorylated Blocker: Because glucose is actively flowing through, the IIAGIC protein remains unphosphorylated.
IIAGIC targets and inhibits LacY (lactose permease) Because LacY is blocked, lactose cannot even cross the cell membrane.
B. Glucose Absent (Bottom Panel: The Green Light)
Phosphates Back Up: When all the glucose runs out, the PTS system stops transporting it, causing phosphate groups to accumulate on the protein chain (HPr, IIA, and IIB).
LacY is Freed: Without the unphosphorylated IIAGIC around to block it, LacY is free to do its job and start importing lactose from the outside
So with no IIAGIC LacY can’t target
The Result: Lactose enters and gets converted to allolactose and triggers the operon to turn on.

Sensing the Environment
Two-component signal transduction
¨Sensor kinase protein
in plasma membrane: This protein sits embedded directly in the cell's plasma membrane
Binds to signal: It acts like an antenna, waiting to bind to an environmental signal such as a food source or a chemical cue.
¨ Food: Binds to food signaland tells the cell there’s food
¨ Chemical cue
Activates itself via phosphorylation
¨Cytoplasmic response regulator
This protein floats freely inside the cytoplasm.
Gets phosphate from sensor: It acts as the messenger's recipient, getting its phosphate group handed over from the sensor kinase
Once activated by that phosphate, it travels to the chromosome and binds to the DNA: Binds chromosome
¨ Alters transcription rate of multiple genes
First food signal binds to outer pocket of sensor kinase,sensor kinase changes shape due to this and grabs a phosphate from ATP, and gives phosphate to repsonse regulator floating in cytoplasm which heads to DNA to turn on needed genes.
so food signal isnt what goes to the cytoplasmis response regulator but the phosphate is what goes
food signal just stays at the sensor kinase protein

Sigma Factor Regulation
§ A regulon is a set of genes and operons scattered around the chromosome with related functions.
- Regulons are coordinately controlled by a single repressor or activator protein.
§ However, in many cases bacteria need to coordinately activate genes, operons, and regulons of seemingly disparate function that are needed for survival.
Normally, individual operons handle specific tasks
when a bacterium encounters a crisis—like a sudden heatwave or toxic stress— it needs to turn on dozens of completely unrelated genes at the same time
- One way to do this is to first regulate the synthesis or activity of the sigma factor that directs the expression of all those genes.
sigma factor lights up everything at once
Altering Transcription Rates
sigma factor guides RNA polymerase to initiate transcription at promoter
¨Proteins can help guide sigma factor to promoter
Activator—The Helper: An activator protein binds to a specific DNA site right next to the promoter.
Binds to DNA sites next to promoter: The Result: Instead of just letting RNA polymerase wander by chance, the activator helps recruit or guide the sigma factor/polymerase complex to the site
Increases frequency of that gene’s transcription
¨Proteins can block sigma factor from binding: The Result: Instead of just letting RNA polymerase wander by chance, the activator helps recruit or guide the sigma factor/polymerase complex to the site
Repressor ¨ Binds to DNA sites next to promoter § Operator
Lowers frequency of that gene’s transcription