MT1 Fricker- Chromosomes, chromatin and 3D organisation of the nucleus
 Call Kai
 Learn
 Practice Test
 Spaced Repetition
 Match
 Flashcards
 Knowt Play
1/5

There's no tags or description
Looks like no tags are added yet.
Name | Mastery | Learn | Test | Matching | Spaced | Call with Kai | Chat |
|---|
No analytics yet
Send a link to your students to track their progress
6 Terms
how did the eukaryotic nucleus originate?
the hydrogen/syntrophy hypothesis:
metabolic symbiosis between an archaeal host and an alpha-proteobacteria leads to gene transfer to the host
the nuclear envelope might have formed to separate transcription from translation- either to protect the dna from reactive oxygen species (from the mitochondrion) or to ensure translation doesn’t start without introns being spliced out
the inside-out hypothesis:
instead of an endosymbiosis event, engulfment via protrusions occurred, in a manner that could lead to nuclear pore and endoplasmic reticulum formation (with the mitochondria escaping from this ER)
the developed syntrophy hypothesis:
in this ecological system, cyanobacteria were producing oxygen needed for the mitochondria, but the archaeal host need a more anoxic environment (for methane metabolism)
a third organism, a delta-proteobacteria could have been the true host, which engulfed both the alpha-protobacteria that became the mitochondrion, and the asgard archaea that became the nucleus within this host
(supporting evidence- asgard archaea could not be cultured without also coming with two other organisms in some syntrophy, and they have histones + SMC proteins)
these theories could be combined together

why do eukaryotes have so much dna?
the presence of the mitochondria, and its increase in efficiency due to genome reduction, permitted a massive increase in the number of genes that could be expressed due to increased energy availability
this increased innovation of the protein folding toolkit
the mitochondria were a prerequisite to this level of complexity and genome size
how are chromosomes organised in bacteria and archaea?
bacteria has a ‘bottlebrush model’ nucleoid (supercoiled loops radiate out from a dense core)- no histones but the chromosome is organised via stable maintenance of chromosome (SMC) proteins
archaea have histones as well as SMC proteins- this supports the idea that archaea were a precursor to the nucleus as we know it

how are chromosomes organised in 3D within the nucleus?
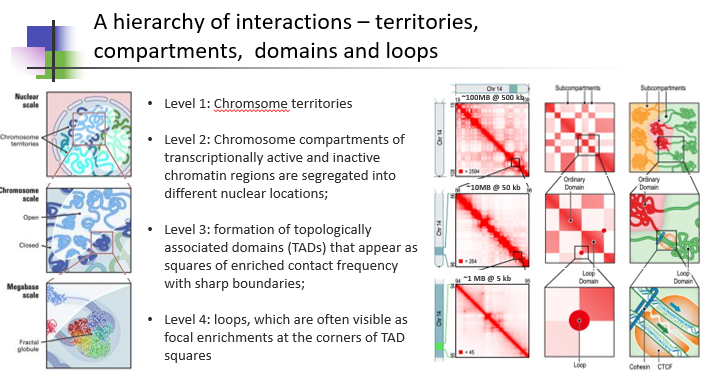
in order of decreasing scale:
level 1: there are distinct chromosome territories within the nucleus but these are not constant/are somewhat ambiguous
level 2: the chromosomes are least active nearest the nuclear envelope (in transcriptionally silent laminar associated domains of chromatin, LADs)- this seems counterintuitive because it means mRNA have to travel further to leave the nucleus, but it may be a method of UV protection
level 3: topologically associated domains (TADs) form between chromosomes, partitioning the nucleus into distinct co-regulatory units (multiple promoter/enhancer/repressor complexes)
level 4: chromosome loops of transcriptionally active regions
how are chromosome loops formed?
cohesin (an SMC protein) can bind tethered DNA and extrude a loop of DNA through the ring, actively driving the movement using ATP hydrolysis
the ring is big enough for nucleosomes to remain bound at their original locations
this is a self-organising system, the extrusion is stopped by convergent CTCF binding:
CCCTC binding factor (CTCF) can recognise and bind two CCCTC motifs 50-60 bases apart in the DNA
this CTCF stalls extrusion of the loop until the SMC is unloaded

why and how is DNA organised into functional clusters in the nucleus?
loops of transcriptionally active DNA are formed through extrusion by SMC proteins
these are clustered into topologically associated domains (TADs) within/between chromosomes based on similar function
this increases efficiency in transcription, because the transcription machinery stays stationary while the DNA moves, and so clustering genes near the machinery increases firing frequency