Immuno Test 4 - Memory
 Call Kai
 Learn
 Practice Test
 Spaced Repetition
 Match
 Flashcards
 Knowt Play
1/25

There's no tags or description
Looks like no tags are added yet.
26 Terms
After the infection has cleared (little to no replicating pathogen) most effector cells die…
but not all…
CD4/8 goes down but ab stays relatively high, they are very stable
Th1 cell cytokine secretion
th1 cells produce IFN-gamma and CD40L which induce and activate M1 macrophages
Fas ligand and LT-beta produced by th1 cells induces the apoptosis of macrophages taken over by bacteria
IL-2 made by th1 cells acts on naive t cells (CD4/8)
IL-3 and GM-CSF made by th1 stimulates production of macrophages in bone marrow
make TNF-alpha and LT-alpha to let macrophages through vessel walls
make CCL2 to guide macrophages (chemotaxies)
Th2 cell cytokine secretion
they make…
IL-13
increases smooth muscle contraction to expel worms (gi tract) and it repairs epithelial cells and mucus (helps shed parasitized cells)(mucus prevents adherence)
IL-4/IL-13
recruit and activate m2 macrophages
IL-5
recruit and activate eosinophils
IL-3/9
mast cell recruitment, use specific IgE to arm them against helminths
Th17 cell cytokine secretion
IL17/22
production of antimicrobial peptides by epithelial cells
IL-22
epithelial cell turnover
IL-17
activates stromal cells and myeloid cells to make G-CSF to stimulate neutrophil production in bone marrow
and recruits neutrophils
CCL20
chemoattractant for other th17 cells
upregulate defensins, go cell turnover stops attachment of bad guys
t effector cell exhaustion
90% die
• Chronic stimulation through the TCR upregulates FAS
• Not enough survival signal (IL-2) to go around
• Metabolic overload
• Maintains niche availability for different T cell dependent responses → if there was no contraction phase there would not be enough il2 or room for new b cells
FAS/FASL pathway
extrinsic cell death pathway
FasL (fas ligand) binds to fas
death domains (protiens) cluster in cytoplasmic side of fas (part of fas), then recruits FADD
recruits pro-capsase 8
plasma cell exhaustion
• ER stress/metabolic stress is primary
• Lack of survival cytokines (IL-7)
But bone marrow is fairly rich
Some survive and continue to secrete antibodies
Secondary exposure to the same/similar pathogen…
induces a more robust and rapid response!
There is a natural contraction of T/B cell numbers following exposure and clearance
right after first exposure can be exposed again and not get sick (this is not the “secondary infection”)
Immunological Memory - maintenance of memory is probably…
antigen-independent but there is evidence that some pathogens are kept in the lymph for a long time (constant low level b cell stimulation)
differences between the primary and secondary immune responses
primary
small amount of pathogen specific cells respond at the start, delay before the pathogen specific antibodies are produced
non isotype switched antibodies have a mixture of affinities
high threshold of activation
delay before effector t cells are generated and are able to enter infected tissues
have to wait for adaptive response
secondary
large number of pathogen specific cells respond immediately and pathogen specific antibodies present
antibodies are isotype switched and have high affinity for pathogen
lower threshold of activation
effector t are present in tissue not just lymph
close cooperation with innate and adaptive from the start
how is memory established during clonal expansion
naive t cell is activated by dc, clones of t cell are made as pathogen specific in effector and memory versions but effector cells out number memory
effector Head to the site of infection: most die after ~5 days, memory remain
naive b cell is activated by pathogen/tfh cell and clones are produced. some memory most plasma. Head to the bone marrow: can be long-lived, but most die after ~5 days
secondary response isotypes, affinity, hypermutation
less igm bc more class switch
higher antibody affinity
higher somatic hypermutation
existing high affinity abs shut down naive weaker b cells
fc receptors are expressed on naive and effector b cells, when high affinity antibodies bind to antigens they interact with these and send an off signal for weaker b cells
some pathogens mimic and exploit this
All secondary responses increase the
concentration of…
Ag specific Abs and the affinity
• Also see an increase in additional
isotypes, but IgG is usually
measured first
Because B cells undergo SHM to improve
Ab binding…
there needs to be a mechanism to inhibit both naïve and less effective B cells
Because the body now possesses upgraded, highly effective memory B cells from that first encounter, it does not want to waste energy activating brand-new naïve B cells that only make weaker, low-affinity antibodies
2. Secondary Response (Naïve B Cells): Pre-existing antibodies coat the returning pathogen and bind to the naïve B cell's inhibitory receptor (FcγRIIB1). This triggers a negative signal that blocks the cell from activating and prevents the production of weak IgM antibodies.
3. Secondary Response (Memory B Cells): Experienced memory B cells bind the pathogen with their upgraded receptors, receiving a positive signal to activate and rapidly produce strong, high-affinity IgG antibodies.
B cell memory is…
less complex than T cell memory
naive vs effector vs memory t cell
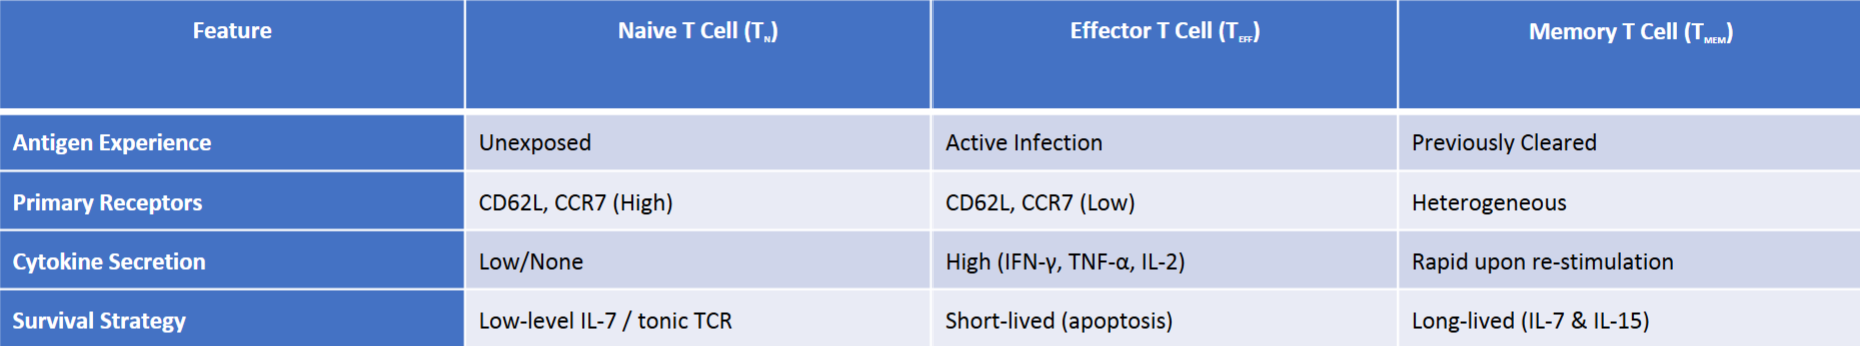
types of memory T cells
Have different requirements for survival, location and longevity
Naïve and memory T cell have different requirements for survival
naive
Naïve T cell require contact with MHC+self peptides for survival (like positive selection in the thymus)(too weak to activate the T cell)
Antigen encounter (signal 1) plus co- stimulation (signal 2) activates the T cell
(proliferation and differentiation)
memory
Memory cells can come directly from the activated naïve cells or from the effector cells
Memory cells need cytokines but not contact with MHC+peptide for survival. This is
different from the naïve T cells (top panel)
Memory T cells need MHC+self peptide to proliferate (weak interactions). These remain memory T cells and do not become effectors until they bind the MHC+the correct foreign peptide (strong binding).
Two important types of T cell memory for this class
TEM become TRM once they enter and stay in the tissue, if they stay circulating TEM

memory t cell development models
Linear Differentiation Model:
Naive (TN) → Effector (TEFF) → Effector Memory (TEM)
→ Central Memory (TCM)
Most effector T cells die during contraction; surviving cells gradually upregulate memory features.
Asymmetric Cell Division Model:
Upon initial APC binding, proximal daughter cells receive higher signal strength (effector fate), while distal daughter cells maintain stem-like properties (memory fate).
Self-renewal Model:
TCM TEM TEFF The reverse of the linear differentiation model
Progressive Differentiation / Decreasing Potential
Model:
Cumulative TCR signal strength and duration dictate cell fate: weak stimulation favors TSCM/TCM, whereas strong/prolonged stimulation drives terminal TEFF
exhaustion. Mix of linear and asymmetric models
TCM reservoir of Ag-specific T cells
• Circulate into and out of lymph nodes to sample antigen
• Very high proliferative capability
Stem cell like—some scientists call them stem cell memory T cells
TEM → TRM rapid responders
• Circulate and then enter the tissue
• Activated upon re-infection
Require very little antigen
No requirement for costimulation
Effector function is pre- programmed
• Do no proliferate
Memory CD8 T cells do not survive without…
the help of CD4 cells
what are vaccines made of….. and why in doses
killed or disassembled viruses
adjuvants (activate innate immune so that can activate the adaptive one, virus is weak and unreplicationg so wont do this by itself)
preservatives, antibiotics
in doses because of somatic hypermutation for b cells → produce a higher affinity ab
central and effector memory
central hangs around in lymph bc CCR7 binds to CCL21/19
effector does not like lymph so downregulates CCR7 + L-selectin
effector memory are already…
differentiated and have effector molecules (central memory dont)