Hon Molecular Exam 2
 Call Kai
 Learn
 Practice Test
 Spaced Repetition
 Match
 Flashcards
 Knowt Play
1/85

Earn XP
Description and Tags
Chromatin, Bacterial Transcription, Eukaryotic Transcription
Name | Mastery | Learn | Test | Matching | Spaced | Call with Kai | Chat |
|---|
No analytics yet
Send a link to your students to track their progress
86 Terms
chromatin
DNA+Protein used as a packaging mechanism for chromosomes
bacterial chromatin
*nucleoid
NAPs
DNA Supercoiling
does bacterial chromatin have histones
no! they use NAPs as a substitute
eukaryotic chromatin
dna double helix
dna wrapped in histones → forms nucleosomes
nucleosomes coiled into a chromatin fiber
futher condensation
mitotic chromosome
histones
small basic proteins rich in Lysine (K) and Arginine (R)
they are both basic and positively charged
allows histones to interact with negatively charged phosphate backbone of DNA
Core histones
H2A, H2B, H3, H4
2 copies of each
A core nucleosome contains ~_____ bp of DNA wrapped around a histone octamer
146
H1
Linker histone, not part of core octamer
Lysine + Argenine make up more than ___ of histone composition (percentage)
20%
histone variants
CENP-A → in centromeres → replaces H3 in nucleosomes, provides platform for kinetochore assembly and chromosome segregation
H2AX → at sites of DNA Damage → phosphorylated at Ser139, marks DNA break regions and helps recruit repair factors
H2AZ → inactive chromatin → associated with active gene expression
nucleosome
basic unit of eukaryotic chromatin (bundle of 8 histones)
centromere (specialized heterochromatin)
responsible for cells ability to properly segregate sister chromatids during cell division
specifically linked to CENP-A
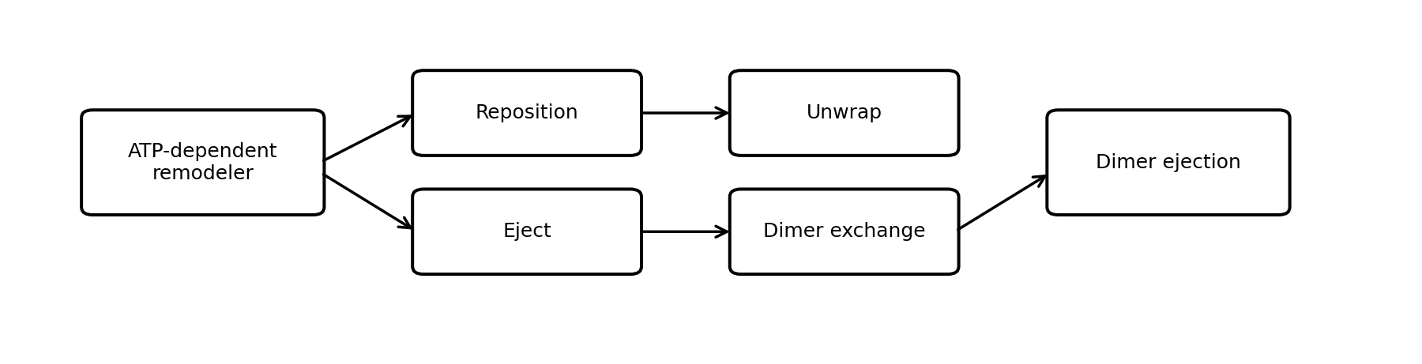
chromatin remodeling
uses energy from hydrolysis of ATP to alter chromatin structure
uses large protein complexes
repositioning: slides nucleosome so DNA binding site is exposed
ejection: removes nucleosome
unwrapping: poses DNA (transient/reversible
dimer exchange: swaps a histone dimer (alters composition)
dimer ejection: removes a dimer (alters composition)
euchromatin (OPPOSITE FOR HETEROCHROMATIN)
transcription: active
nucleosome density: low, open, depleted
DNA Methylation: low
histone acetylation: high
histone methylation: low
H3K4 methylation: high (exception)
H3K9/H3K27 methylation: low
5-Methylcytosine
5-mc
generally associated with transcription repression
methylated at transposable elements and gene body
unmethylated at promoters
DNA methylation
adding a methyl group to suppress/turn off gene activity
both in bacteria and eukaryotes
protects against cleavage of their genomes by restriction enzymes
E.Coli methylation
E.Coli has a methyl transferase enzyme called DAM that methylates DNA
methylates A in sequence GATC
types of histone covalent modifications
acetylation (KST)
methylation (KR)
phosphorylation (STYHD)
eukaryotic acetylation
KST
frequently found at the promoters and enhancers of active genes → associated with activation of gene
lysine acetylated by histone acetyltransferases (HATs)
lysine removed by histone deacetylases (HDACs)
neutralizes lysines positive charge → weaker histone = more accessible chromatin
eukaryotic methylation
KR
H3K4 methylation → high in euchromatin, found at enhancers and promoters
H3K9/H3K27 methylation → high in heterochromatin, found upstream of silent genes
H3K36/H3K79 methylation → found at bodies of active genes
Creates binding sites for reglatory proteins, usually associated with repression
eukaryotic phosphorylation
STYHD
H2AX: Phosphorylation on serine 139 is a characteristic of sites of DNA Breakage
phosphorylation cascade
phosphorylation cascade
major means by which the cell responds to extracellular signals
signal → kinase activation → phosphorylation of next protein → more phosphorylation → altered regulator activity → altered gene expression
x-inactivation
inactivation of one copy of the x chromosome in female cells
one x chromosome is inactivated by XIST (functional noncoding RNA)
XIST leads to the recruitment of factors that methylate H3K9/H3K27 and DNA
Murray Barr + Ewart Bertram 1948
in female cats, neurons found a darkly stained spot in the nucleus
condensed inactive X is called a Barr body
Susumu Ohno 1959
one x-chromosome was darkly stained → marker of heterochromatin
barr body should look like heterochromatin (transcriptionally repressed, high methylation, enriched for repressive histone methylation)
Mary Lyon 1961
proposed that inactivation is random
mx and px are equally likely to be silenced → lyonization
hox gene
specify body plan in multicellular organisms
present in every cell but expressed differently in each
must be expressed in the righ cell types and silenced everywhere else
polycomb gene (PcGs)
represses scr expression in middle + hind legs so sex combs only form on front legs of male flies
found to catalyze H3K27me3 (methlation of H3K27 → repression)
trithorax gene
activates scr gene in front legs
if mutated, scr expression is reduced in front legs
catalyzes H3K4me3 which is an exception and is associated with active gene transcription
can also catalyze H3K27ac (acetylation of H3K27)
bacterial transcription basics
first step in flow of genetic information
DNA-Dependent RNAP
catalyze formation of phosphodiester bonds → hydrolysis of phosphodiester bonds is unlikely because of pyrophosphate hydrolysis which releases a lot of free energy
(RNA-Dependent RNAP used for RNA interference not transcription)
nascant RNA only grows 5’ to 3’
RNAP's do not require a primer
Exception: reverse transcription by retroviruses (HIV)
RNAP core enzymes (sufficient for RNA synthesis)
a - complex assembly
a - complex assembly
b - forms “pincer”, contains rifampicin-binding pocket (inhibitor)
b’ - forms “pincer”, catalytic subunit
omega - complex assembly
RNAP holoenzymes
a - complex assembly
a - complex assembly
b - forms “pincer”, contains rifampicin-binding pocket (inhibitor)
b’ - forms “pincer”, catalytic subunit
omega - complex assembly
sigma - recognizing promoters (required for initiation), ejected during elongation
transcription promoters
required, must be upstream
consensus sequences: derived from alignments
-35
-10
mutations: changing spacing between boxes usually decreases transcription but can potentially increase it
Methods for discovering promoter boxes
DNase Protection Assay
incubate RNAP holoenzyme with a DNA fragment containing a promoter
isolate protected fragment and determine its sequence
DNase 1 footprinting technique
a bound protein leaves a footprint
gap in the cleavage ladder reveals the exact protected region
sigma factor
recognizes specific promoters and is required for the initiation of transcription
sigma 70 aka sigma D : major sigma factor during exponential growth
sigma 54 aka sigma N: nitrogen metabolism genes
bacterial initiation : RNAP promoter complex
RNAP holoenzyme recognizes promoter and forms a closed complex
closed complex: DNA strand stays together
DNA melts are the staert site and forms the open complex
open complex: DNA strand separates
permanganate footprinting: attacks single-stranded DNA only
bacterial initiation continued
RNAP scrunches downstream DNA (8-10 nt)
open complex formed
accumulation of enough energy from scrunching allows promoter to escape → productive elongation
sigma factor is ejected
bacterial elongation
NTPs reach catalytic site and provide the chemical energy for chain extension
drives RNAP downstream
RNAP pauses during elongation because it does not always move at a fixed rate
can pause and backtrack
mismatched DNA is cleaved (cut): GreA and GreB enhace cleavage allowing a corrected 3’ end to re-enter active site and resume elongation
bacterial termination
Instrinsic
GC-rich inverted repeat → RNA stem loop → causes RNA to pause
approx 8-10 U-rich residues → improtant for release of nascent RNA chain
Rho-Dependent
C-rich rho utilization (rut) site in RNA + Rho Factor
polycistronic mRNA
multiple protein-coding sequences with one promoter
common in prokaryotes, rare in eukaryotes
monocistronic mRNA
single protein chain
common in eukaryotes
operon
segment of DNA containing multiple genes regulated by a single promoter
polycistronic
Jacques Monod + Francois Jacob 1960
performed experiments to understand how the genes in E.Coli allowing lactose to metabolize lactose are regulated
used constitutive mutants to make lac mRNA regardless of presence of lactose
they made partial diploids because E.Coli is haploid
found mutations LacI and LacO
lac operon composition
promoter, operator, LacZ, LacY, LacA
lacZ, LacY, and LacA are in high levels with high lactose medium until they account for 1% of total protein in cell (Inducible)
mutations: LacI, LacO
official order: laci, laco, lacz, lacy, laca
lacL (mutation)
encodes the diffusible LacI repressor
recessive: partial diploids wiht one good copy of LacI showed inducible synthesis
when lactose is present, LacI is not at operator
LacOc (mutation)
operator
DNA site bound by LacI
cis-acting regulatory element
“c” = constitutive
can cause constitutive synthesis of lac mRNA only when it is on the same DNA molecule as lacZ+
constitutive if it has LacOc/LacZ+ somewhere ***
inducible if not
LacZ
B-Galactosidase
breaks lactose into galactose and glucose
inducible
LacY
Lactose permease, imports lactose
inducible
LacA
B-galactoside transacetylase
CRP site
binds cAMP-CRP activator when glucose is low
when glucose is present, cAMP-CRP activator is not
which is preferred: glucose or lactose
glucose!!
if there are high levels of Trp…
RNAP is terminated and mRNA is not extended
does not want to make more tryptophan, wants to use from environment if possible
ribosome does not stall at tandem trp codons → 3-4 terminator forms → terminates early → trp gene OFF
if there are low levels of trp…
ribosome stalls at tadem Trp codon → 2-3 antiterminator forms → continues transcription → Trp gene ON
TrpR
on/off switch for repressor system
decreases transcription ~70-fold
Attenuation
A sequence of 28 bases in the leader
provides finer control
decreases transcription ~10-fold
similarities between bacterial and eukaryotic transcription
large multi-subunit RNAPs
need a promoter for initiation
regulated by DNA binding proteins
differences between bacterial and eukaryotic transcription
eukaryotic transcription has multiple RNAPs
eukaryotic has more initiation factors
eukaryotic has nucleosomes (histones)
RNAP I (euk)
encodes rRNA
RNAP II (euk)**
encodes mRNA, incRNA, miRNA, etc…
RNAP III (euk)
encodes tRNA
RNAP VI (euk)
encodes siRNA (only in plants!)
eukaryotic protein-coding gene structure
regulatory promoter upstream of a core promoter, followed by 5’-exons and introns-3’
exons: protein coding regions
introns: non-protein coding regions that break up exons
core promoters
TATA box
BREs (2)
Inr
DPE
Assembly of PIC in correct order
core promoters: BRE - TATA box - BRE - Inr - DPE
GTFs: TFIID → A > b → F Pol II → E → H
TATA box
bound by TBP (subunit of TFIID) to initiate PIC formation
only 10% of promoters in any eukaryotic genome have TATA boxes
BREs
TFIIB response elements, bind TFIIB
Inr
initiator element near the transcription start site
DPE
Downstream promoter element
TAFs
TBP-associated factors that allow TFIID to recognize Inr/DPE in absence of TATA box
TFIID
contains TBP and 13 TAFs
contains Inr and DPE
scaffold for PIC, integrates regulatory signals
Regulation of TBP
T1/2 > 1Hr
persistent binding of TBP could result in over-activation
solution: Mot 1 - enzyme that removes TBP from DNA
TFIIA
after TFIID
stabilizes binding of TBP and TFIID to the core promoter
TFIIB
after TFIIA
binds BREs
stabilizing binding of TFIID to core promoter
helps recruit the RNAP II - TFIIF complex (next)
participates in selection of transcription start sites (TSSs)
TFIIF-Pol II
recruited along with RNAP II
necessary for TFIIE/TFIIH recruitment
participates in TSS selection
TFIIE
after TFIIF
helps recruit TFIIH
necessary for promoter melting
TFIIH
last GTF
acts as helicase and unwinds DNA to form open complex
phosphorylates RNAP II CTD
regulatory promoters
upstream of core promoters
bound by specific activators
regulatory enhancers
distance-independent
orientation-independent (forward or backward)
contains specific protein-binding sequences
acts by looping to target promoters
SV40
study of SV40 transcription revealed two identical sequences upstream of reg. promoter
removal of one → small inhibition of transcription
removal of both → transcription stopped completely
enhancer is not specific not SV40
Can be inserted forwards OR backwards
insulators
mediated by CTCF protein
blocks enhacer activity and/or creates a boundary between euchromatin and heterochromatin
activators
two domains:
DNA-binding domain → recognizes specific sequences in promoters and enhancers
activation domain → contacts transcription machinery
uses two-hybrid assay in lab
mediator
bridge between transcription activators and RNAP
required for euk transcription
head and middle: contact RNAP II
tail: contacts activator
reporter assays
used to test the strength and activity of a promoter
common examples:
green flourescent protein (GFP)
LacZ (blue pigment used in cloning)
eukaryotic elongation
C-terminal domain must be phosphorylated
RNAP II has regulated pausing
regulated by NELF and DSIF (negative charge)
pause released by P-TEFb (positive charge)
stalled/backtracked RNAP II is rescued by TFIIS
nucleosomes represent impediments to RNAP II progress
FACT (facilitates chromatin transcription)
FACT
allows RNAP II to transcribe through packaged DNA
removes a single dimer of H2A-H2B ahead of RNAP→ loosens packaging
reassembles nucleosome behind RNAP by returning missing histones
eukaryotic termination
RNAP I : TTF-1 recognizes a specific sequence in rRNA genes and blocks further transcription
RNAP II : No single specific termination seuqence mentioned ; requires RNA processing
RNAP III : Transcripts have ~4-7 Us at the 3- end → triggers RNAP III release